Lecture 6: Natural Selection I: Adaptation#
Natural selection is perhaps the primary organizing principle in evolution. One knows this intuitively; look out your window (or if it’s pouring rain in Eugene, which let’s face it it probably is, pull up a nature documentary) and what you will see are a collection of organisms who are supremely well adapted to their environments. Natural selection has shaped all of life, from biochemicals and genomes to phenotypes and perhaps even species.
While this is so one must be very specific when defining or deciding that one is actually “looking at” an adaptation or that something is adapted. The issue revolves around the general belief that the environment presents problems for the organism and that adaptations provide solutions to these problems.
What is an adaptation?#
First let’s clarify some terminology. The word Adaptation comes from Latin ad (to, towards) and aptus (fitted). But it is important to distinguish different uses of the word “adaptation” in the biological sciences. An adaptation in physiology is a change in response to a certain problem: you heat up and respond by taking off your jacket (a behavioral “adaptation” to an environmental problem); you continue to heat up and respond by sweating (a physiological response to an environmental problem).
In an evolutionary context: also a change in response to a certain problem. This time the change is genetic, is achieved by the process of natural selection and takes place over a period of time considerably longer than the physiological time scale. But note: the physiological response itself could be an “adaptation” in the evolutionary sense: it can be (is) adaptive (genetically) to adapt physiologically or behaviorally.
The word Adaptation is both a state of being (phenotypic trait or character) and it is a process by which such traits come to be called “adaptations”.
Implicit in the term adaptation is the belief that an adaptation serves some function or purpose. Dispersal and reproduction are the function or purpose of an apple, and apples are an adaptation apple trees use to achieve reproduction. This assumes natural selection led to the apple as the agent of dispersal and reproduction. Avoiding predation is the function or purpose of leaf-like coloration in insects and frogs and their coloration is an adaptation these insects use to avoid predation.
As argued by G. C. Williams in his classic book Adaptation and Natural Selection (1966), it is important to distinguish adaptations from “effects”: an effect of being an apple is to provide food for insect larvae or humans; food is an effect of an apple’s phenotype (good resources); apple farming is an effect of apples’ good taste and nutritional value (apples did not evolve to solve the problem of providing work for apple farmers); the cryptic coloration of a katydid is not for the purpose of demonstrating adaptation in evolution lectures; demonstration is an effect of the striking morphology.
To reiterate: we identify traits as adaptations only when they evolved for the solutions of a specific problem (function/purpose).
Selection is myopic#
Evolution produces some really clear trends, and presumably they’re adaptive. Some trends lead to intensification of a character, like the ever bigger horns, antlers, and other weapons that males use in fighting and displaying for females. Other trends go the other way and lead to diminution. Fleas lost their wings, which makes sense for an animal that makes its living crawling down through the hair of its host to get at the skin. Cave animals like the blind Mexican cavefish (Astyanax mexicanus) lose their eyes and pigment. The important thing is that selection doesn’t have a “goal” of bigger antlers or no eyes or smaller wings in mind. Selection is myopic. It only sees whether a slightly bigger antler or a slightly smaller wing does better right now, in this generation, and the trend is just what adds up when that keeps happening over and over.
Also be careful even with those examples! It’s tempting to say that cavefish lost their eyes because making eyes is expensive, so fish that didn’t waste energy on useless organs had higher fitness. That’s one hypothesis. But it could also be that once you live in total darkness there is no selection keeping the eyes working, so mutations that break eyes just drift around and pile up. Or the genes that make eyes might do other things too (pleiotropy, remember?), and selection on those other things drags the eyes along. People have been testing these ideas in cavefish for years, and it looks like more than one of them is going on.
Exaptation#
Now we have a problem of identifying adaptations in this context. Many traits evolved under one selective regime and are now being used under a very different selective regime. The current function may not reflect the context in which a trait evolved. We have to be able to distinguish current utility from historical origin. Some traits may have evolved in one context but later such a trait may be co-opted for use in a different role. One term used to refer to such traits is Preadaptation. Some evolutionary biologists dislike this term (some get nauseous when they hear it!) because the term implies that an adaptive trend was anticipating some future need. We know that evolution is “blind”, “shortsighted” and can’t foresee or anticipate new selective regimes. Key point is that a trait’s function can change faster than its form.
S.J. Gould and E. Vrba (1982) have suggested a different term, exaptation, to stress the co-optedness of traits. Here’s the distinction they’re drawing. An adaptation is a trait whose current function is the one natural selection built it for. An exaptation is a trait that is useful now for something other than what it was originally shaped for- either it evolved under selection for some other job, or it wasn’t shaped by selection at all and just happened to turn out useful. Notice the word says nothing about the future, so it gets around the problem with “preadaptation”. Nothing was preparing for anything, a trait just got picked up and put to a new use. And once it’s been co-opted, selection can go on to modify it for the new job too, so plenty of traits are a mix of both.
Feathers are a great example. We now have lots of fossils of dinosaurs covered in simple feathers that clearly couldn’t fly, like Sinosauropteryx (Chen et al. 1998; see Fig. 7). So feathers probably first evolved for something like insulation or display, and were only later co-opted for flight. Feathers are an exaptation for flight, and then selection went to work refining them into the flight feathers we see on birds today.
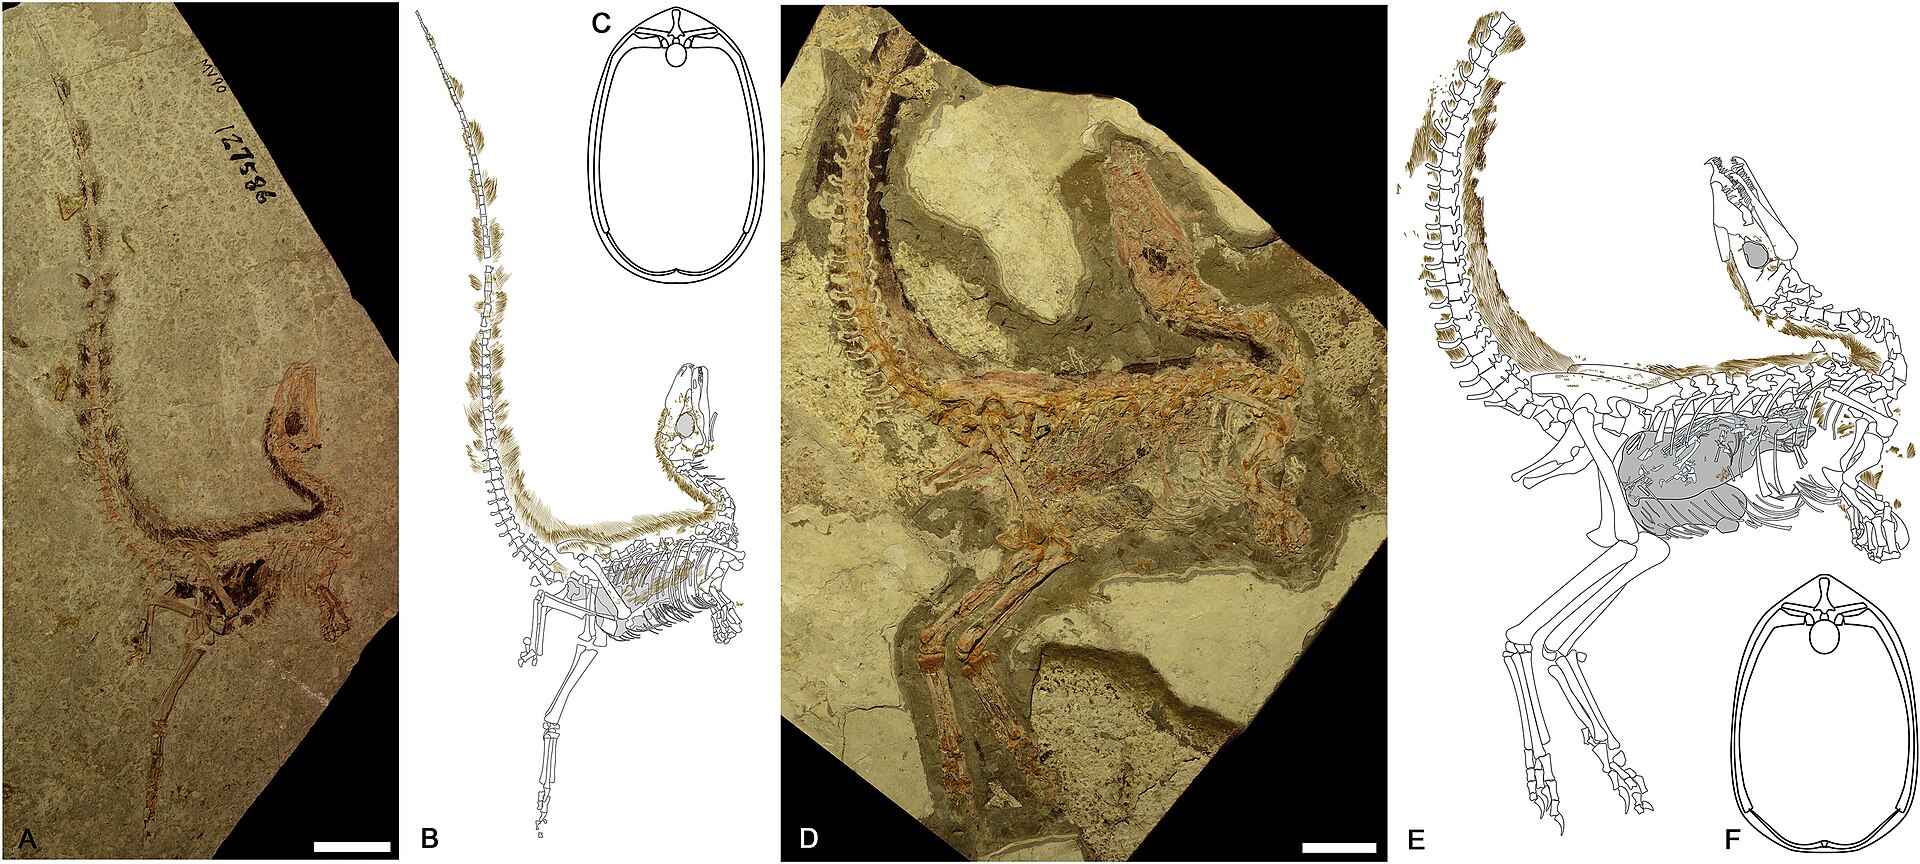
Fig. 7 Feathers on a dinosaur that couldn’t fly. Two fossils of Sinosauropteryx (A and D) with drawings (B and E) that map out where feathers are preserved, shown in brown. Notice the fuzz of simple feathers running all the way down the neck, back, and tail. From Smithwick et al. 2017, via Wikimedia Commons, CC BY 4.0.#

The feathers on these fossils are preserved well enough that we can even tell what color the animal was! The feathers still contain melanosomes, the little packets of pigment inside cells, and their shapes and positions tell us where the animal was dark and where it was light. Smithwick and colleagues used them to reconstruct Sinosauropteryx in Fig. 8. It had a reddish brown back and a pale belly (countershading, the same camouflage trick lots of animals use today) and a striped tail.
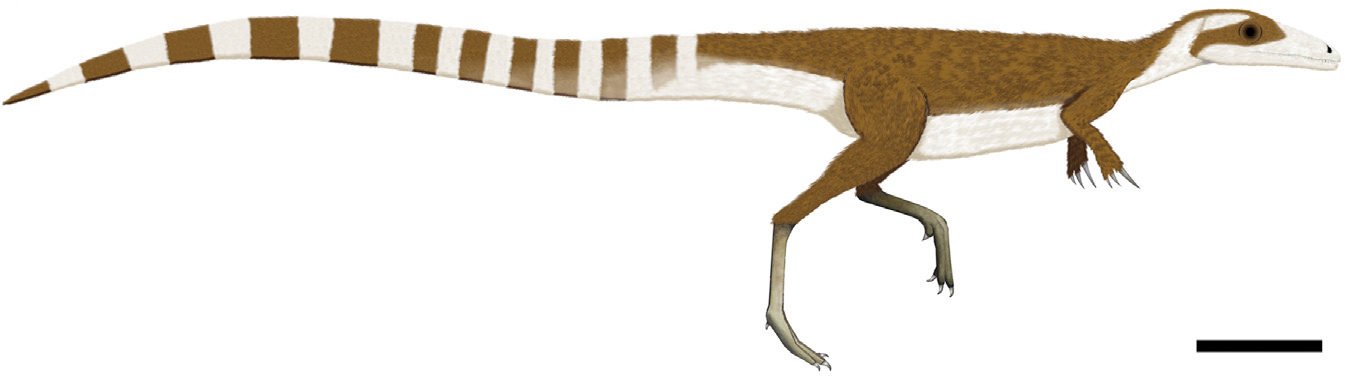
Fig. 8 What Sinosauropteryx looked like, reconstructed from pigments preserved in its feathers. Art by Robert Nicholls, from Smithwick et al. 2017, via Wikimedia Commons, CC BY 4.0.#

Three examples. First, the evolution of bone tissue is believed to have proceeded under selection for a tissue that stores inorganic ions (e.g. phosphate ions). The ions need to be stored and released depending on the physiological demands of the body. The tissue best at doing this became rigid and could be co-opted as a structural member. Thus organisms with “bone” as a structural tissue entered a new “adaptive zone” and adapted for various functions.
Second, skull sutures in mammals. This one is actually Darwin’s own example from the Origin. The sutures look like an adaptation for birth since they allow the skull to deform when passing through the birth canal (a tight squeeze). But reptiles and birds have them too and they hatch out of eggs! So sutures evolved in one context (allowing for growth of the brain and head) but are an exaptation for birth in mammals (they do allow for the head to change shape during birth which is adaptive).
Third, isolating mechanisms, the traits that prevent gene flow between incipient species. These often evolve while populations are geographically separated (in allopatry), before either population has ever run into its sister taxon, so they can’t have evolved for keeping the species apart. Isolating mechanisms may undergo subsequent adaptive changes once the two species come back into contact though (more when we get to speciation). In all these cases the historical origin is quite distinct from the current utility.
Exaptation also allows for the evolution of traits that originally had no “adaptive” function, but later get co-opted for a function.
The adaptationist program and spandrels#
The Adaptationist Program as it has been called by Gould and Lewontin (1979) seeks to find adaptive explanations for every characteristic of the organism. This is the paper we’re reading in discussion section, so read it! The title comes from the cathedral of San Marco in Venice. Where the round arches that hold up the dome meet, there are these curved triangular spaces called spandrels, and in San Marco they are covered in gorgeous mosaics that fit the space perfectly. You’d be tempted to think the whole building was designed to show off those mosaics. But the spandrels are just an unavoidable side effect of putting a dome on top of arches, and the artists made the best of the space they got. Gould and Lewontin argue lots of biological traits are like that- spandrels, side effects of something else, that we then tell adaptive stories about.
So some things are not “for” the “purpose” or “role” they seem to be filling, and some things are just nonadaptive, which is different from maladaptive (former = neutral; latter = bad). Think of your chin; it’s not “for” something. As Gould told it, it’s there because the part of your lower jaw that holds your teeth and the rest of the lower jaw grow at different rates, and the chin is what’s left sticking out. It’s just there. The striking pattern of white triangles on the Conus shell looks like it is “for” something but these snails live under the sand and mud and the pattern isn’t visible. It could be due to the chemistry of shell deposition or might have been “useful” in the shell’s ancestor.
Phenotypes are compromises#
Another important point against the Adaptationist Program is that some traits may not be capable of achieving “maximal adaptedness”. Selection acts on the entire phenotype (though this is debatable, see units of selection later), and so phenotypes are compromises. A nice example is central place foraging (Orians and Pearson 1979). Think of a bird that has a nest in the middle of its territory and flies out to collect food and bring it back. You could work out the optimal foraging strategy for how far to fly and which food items to go after based on how big they are and how far away. BUT, when the bird leaves the nest, its young are exposed to predators. So the foraging strategy we actually see might not be the best foraging strategy, but the best compromise given predation risk. Or think of green sea turtles. They are excellent swimmers, but terrible diggers (flippers weren’t built for it), yet females must use their flippers to dig a hole for laying eggs. Flippers are not “optimal” for digging, but they work.
Phenotypes as compromises underscores the importance of constraints. Evolution of one trait can be constrained due to genetic correlations among traits, often because the same genes affect more than one trait (pleiotropy again!). Some classic examples from breeding: selection for body weight in broiler chickens gets you more fat along with it; selection for increased milk yield in cows gets you more milk, but with a higher water content; selection for yield in soybeans gets you less protein per bean; selection for nicotine content in tobacco and tar content increases. These are artificial selection examples but the same thing applies to natural selection as well.
Constraints can be phylogenetic or developmental. It might be adaptive for certain mammals to be able to breathe under water, but their phylogenetic history and developmental program constrains them from evolving gills. Instead seals and whales “solve” this “problem” by carrying their oxygen with them. They have huge blood volumes and tons of myoglobin (the oxygen storing protein) packed into their muscles (Mirceta et al. 2013), and when they dive their heart rate drops way down to save oxygen (the diving response). That way most of their dives never run out of oxygen at all.
How do we study adaptation?#
An informative means of analyzing adaptations is through the comparative approach, comparing lots of species to see whether a trait goes along with a particular environment or way of life. But it’s wise to put adaptations in a phylogenetic context. Closely related species tend to share traits simply because they inherited them from a common ancestor, not because each one adapted independently, so we can’t treat every species as an independent data point (Felsenstein 1985). Take rhinoceros horns. Some rhino species have one horn and some have two, with different shapes and sizes. Is each pattern uniquely adaptive for that species? Or are they just neutral variations around a general adaptive theme that happened to get passed down to different lineages? Experiments need to be done to tell those apart (difficult experiments! can you design some?).
Some people have pulled experiments like this off. John Endler’s work on guppies is a classic (Endler 1980). Male guppies in streams with lots of predators are pretty drab, while males in streams with few predators are covered in bright spots. Endler moved guppies from a high predation stream into a stream that had no guppies and only one wimpy predator, and within a couple of years (something like 15 generations) the males there had evolved more and bigger spots. That’s adaptation happening right in front of us, and a real experimental test of what it’s an adaptation to.
In seeking adaptive explanations for phenomena we should also seek parsimonious adaptive explanations. Williams had a great example. A flying fish leaps out of the water, and then it comes back down. We could be adaptationist about it and say the fish evolved the means of returning to the water, but physics offers a much more parsimonious explanation for that- gravity! The interesting problem is not how it comes down, but why it takes so long to do so. Gliding really must be a result of natural selection. Point is: use the simplest explanation that accounts for the existence of a trait. As Williams put it, adaptation is “a special and onerous concept that should be used only where it is really necessary”, and parsimony demands that we recognize adaptation at the level necessitated by the facts and no higher.